Henry David Thoreau

Thank God men cannot fly, and lay waste the sky as well as the earth.

Mohandas K. Gandhi

There is a sufficiency in the world for man's need but not for man's greed.

Robert Orben

There's so much pollution in the air now that if it weren't for our lungs there'd be no place to put it all.

Alan M. Eddison

Modern technology,Owes ecology,An apology.

Henrik Tikkanen

Because we don't think about future generations, they will never forget us.

Showing posts with label in. Show all posts

Sunday, October 14, 2012

Overexploitation in aquatic ecosystems

              Marine biodiversity loss, largely through overfishing, is increasingly impairing the capacity of the world’s oceans to provide food, maintain water quality, and recover from perturbations (Worm et al. 2006). Yet marine fisheries provide employment and income for 0.2 billion people around the world, and fishing is the mainstay of the economy of many coastal regions; 41 million people worked as fishers or fish farmers in 2004, operating 1.3 million decked vessels and 2.7 million open boats (FAO 2007). An estimated 14 million metric tons of fuel was consumed by the fish-catching sector at a cost equivalent to US$22 billion, or ~25% of the total revenue of the sector. In 2004, reported catches from marine and inland capture fisheries were 85.8 million and 9.2 million tons, respectively, which was worth US$84.9 billion at first sale. Freshwater catches taken every year for food have declined recently but on average 500 000 tons are taken from the Mekong river in South-East Asia; 210 000 tons are taken from the Zaire river in Africa; and 210 000 tons of fish are taken from the Amazon river in South America. Seafood consumption is still high and rising in the First World and has doubled in China within the last decade. Fish contributes to, or exceeds 50% of the total animal protein consumption in many countries and regions, such as Bangladesh, Cambodia, Congo, Indonesia, Japan or the Brazilian Amazon. Overall, fish provides more than 2.8 billion people with ~20% or more of their average per capita intake of animal protein. 

             The oscillation of good and bad years in marine fisheries can also modulate the protein demand from terrestrial wildlife populations (Brashares et al. 2004). The share of fish in total world animal protein supply amounted to 16% in 2001 (FAO 2004). These ‘official’ landing statistics tend to severely underestimate catches and total values due to the enormous unrecorded contribution of subsistence fisheries consumed locally. Although the world’s oceans are vast, most seascapes are relatively low-productivity, and 80% of the global catch comes from only ~20% of the area. Approximately 68% of the world’s catch comes from the Pacific and northeast Atlantic. At current harvest rates, most of the economically important marine fisheries worldwide have either collapsed or are expected to collapse. Current impacts of overexploitation and its consequences are no longer locally nested, since 52% of marine stocks monitored by the FAO in 2005 were fully exploited at their maximum sustainable level and 24% were overexploited or depleted, such that their current biomass is much lower than the level that would maximize their sustained yield (FAO 2007). The remaining onequarter of the stocks were either underexploited or moderately exploited and could perhaps produce more. The Brazilian sardine (Sardinella brasiliensis) is a classic case of an overexploited marine fishery. In the 1970s hey-day of this industry, 200 000 tons were captured in southeast Brazil alone every year, but landings suddenly plummeted to <20 000 tons by 2001. Despite new fishing regulations introduced following its collapse, it is unclear whether southern Atlantic sardine stocks have shown any sign of recovery.

             With the possible exception of herring and related species that mature early in life and are fished with highly selective equipment, many gadids (e.g. cod, haddock) and other non-clupeids (e.g. flatfishes) have experienced little, if any, recovery in as much as 15 years after 45–99% reductions in reproductive biomass (Hutchings 2000). Worse still, an analysis of 147 populations of 39 wild fish species concluded that historically overexploited species, such as North Sea herring, became more prone to extreme year-on-year variation in numbers, rendering them vulnerable to economic or demographic extinction (Minto et al. 2008). Marine fisheries are an underperforming global asset—yields could be much greater if they were properly managed. The difference between the potential and actual net economic benefits from marine fisheries is in the order of US$50 billion per year—equivalent to over half thevalue of the global seafood trade (World Bank 2008). The cumulative economic loss to the global economy over the last three decades is estimated to be approximately US$2 trillion, and in many countries fishing operations are buoyed up by subsidies, so that the global fishery economy to the point of landing is already in deficit. Commercial fishing activities disproportionately threaten large-bodied marine and freshwater species (Olden et al. 2007). This results in fishermen fishing down the food chain, targeting ever-smaller pelagic fish as they can no longer capture top predatory fish. This is symptomatic of the now widely known process of ‘fishing down marine food webs’. Such sequential
size-graded exploitation systems also take place in multi-species assemblages hunted in tropical forests (Jerozolimski and Peres et al 2003). 

               In the seas, overexploitation threatens the persistence of ecologically significant populations of many large marine vertebrates, including sharks, tunas and sea turtles. Regional scale populations of large sharks worldwide have declined by 90% or more, and rapid declines of >75% of the coastal and oceanic Northwest Atlantic populations of scalloped hammerhead, white, and thresher sharks have occurred in the past 15 years (Baum et al. 2003; Myers and Worm 2003; Myers et al. 2007). Much of this activity is profligate and often driven by the surging global demand for shark fins. For example, in 1997 line fishermen captured 186 000 sharks in southern Brazil alone, of which 83% were killed and discarded in open waters following the removal of the most lucrative body parts (C.M. Vooren, pers. comm.). Of the large-bodied coastal species affected by this trade, several have virtually disappeared from shallow waters (e.g. greynurse sharks, Carcharias taurus). Official figures show that 131 tons of shark fins, corresponding to US $2.4 million, were exported from Brazil to Asia in 2007. Finally, we know rather little about ongoing extinction processes caused by harvesting. For example, from a compilation of 133 local, regional and global extinctions of marine fish populations, Dulvy et al. (2003) uncovered that exploitation was the main cause of extinctions (55% of all populations), but these were only reported after a median 53-year lag following their real-time disappearance. Some 80% of all extinctions were only discovered through historical comparisons; e.g. the near-extinction of large skates on both sides of the Atlantic was only brought to the world’s attention several decades after the declines have occurred.

Sunday, August 12, 2012

Overexploitation in tropical forests

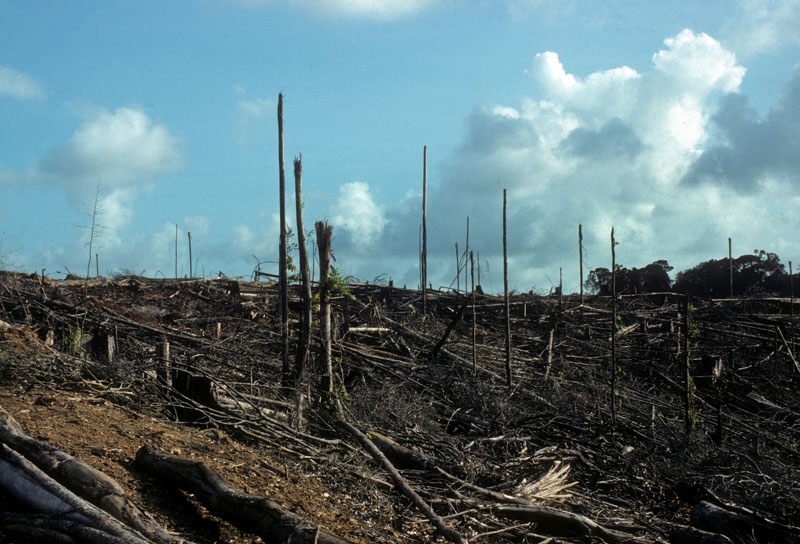
             Tropical deforestation is driven primarily by frontier expansion of subsistence agriculture and large development programs involving resettlement, agriculture, and infrastructure. However, animal and plant population declines are typically pre-empted by hunting and logging activity well before the coup de grĂ¢ce of deforestation is delivered. It is estimated that between 5 and 7 million hectares of tropical forests are logged annually, approximately 68-79% of the area that was completely deforested each year between 1990 and 2005 [FAO (Food and Agriculture Organization of the United Nations) 2007]. Tropical forests account for ~25% of the global industrial wood production worth US$400 billion or ~2% of the global gross domestic product [WCFSD (World Commission on Forests and Sustainable Development) 1998]. Much of this logging activity opens up new frontiers to wildlife and non-timber resource exploitation, and catalyses the transition into a landscape dominated by slash-and burn and large-scale agriculture. Few studies have examined the impacts of selective logging on commercially valuable timber species and comparisons among studies are limited because they often fail to employ comparable methods that are adequately reported. The best case studies come from the most valuable timber species that have already declined in much of their natural ranges.

            For instance, the highly selective, but low intensity logging of broadleaf mahogany (Swietenia macrophylla), the most valuable widely traded Neotropical timber tree, is driven by the extraordinarily high prices in international markets, which makes it lucrative for loggers to open-up even remote wilderness areas at high transportation costs. Mechanized extraction of mahogany and other prime timber species impacts the forest by creating canopy gaps and imparting much collateral damage due to logging roads and skid trails (Grogan et al. 2008). Mahogany and other high-value tropical timber species worldwide share several traits that predispose them to commercial extirpation: excellent pliable wood of exceptional beauty; natural distributions in forests experiencing rapid conversion rates; low-density populations (often <1 tree/ha); and life histories generally characterized as non-pioneer late secondary, with fast growth rates, abiotic seed dispersal, and low-density seedlings requiring canopy disturbance for optimal seedling regeneration in the understory (Swaine and Whitmore 1988; Sodhi et al. 2008). One of the major obstacles to implementing a sustainable forestry sector in tropical countries is the lack of financial incentives for producers to limit offtakes to sustainable levels and invest in regeneration. Economic logic often dictates that trees should be felled whenever their rate of volume
increment drops below the prevailing interest rate (Pearce 1990). Postponing harvest beyond this point would incur an opportunity cost because profits from logging could be invested at a higher rate elsewhere.

            This partly explains why many slow-growing timber species from tropical forests and savannahs are harvested unsustainably (e.g. East African Blackwood (Dalbergia melanoxylon) in the Miombo woodlands of Tanzania; Ball 2004). This is particularly the case where land tenure systems are unstable, and where there are no disincentives against ‘hit-and-run’ operations that mine the resource capital at one site and move on to undepleted areas elsewhere. This is clearly shown in a mahogany study in Bolivia where the smallest trees felled are ~40 cm in diameter, well below the legal minimum size (Gullison 1998). At this size, trees are increasing in volume at about 4% per year, whereas real mahogany price increases have averaged at only 1%, so that a 40-cm mahogany tree increases in value at about 5% annually, slowing down as the tree becomes larger. In contrast, real interest rates in Bolivia and other tropical countries are often >10%, creating a strong economic incentive to liquidate all trees of any value regardless of resource ownership. Tropical deforestation is driven primarily by frontier expansion of subsistence agriculture and large development programs involving resettlement, agriculture, and infrastructure. However, animal and plant population declines are typically pre-empted by hunting and logging activity well before the coup de grĂ¢ce of deforestation is delivered.

            It is estimated that between 5 and 7 million hectares of tropical forests are logged annually, approximately 68-79% of the area that was completely deforested each year between 1990 and 2005 [FAO (Food and Agriculture Organization of the United Nations) 2007]. Tropical forests account for ~25% of the global industrial wood production worth US$400 billion or ~2% of the global gross domestic product [WCFSD (World Commission on Forests and Sustainable Development) 1998]. Much of this logging activity opens up new frontiers to wildlife and non-timber resource exploitation, and catalyses the transition into a landscape dominated by slash-andburn and large-scale agriculture. Few studies have examined the impacts of selective logging on commercially valuable timber species and comparisons among studies are limited because they often fail to employ comparable methods that are adequately reported. The best case studies come from the most valuable timber species that have already declined in much of their natural ranges. For instance, the highly selective, but low intensity logging of broadleaf mahogany (Swietenia macrophylla), the most valuable widely traded Neotropical timber tree, is driven by the extraordinarily high prices in international markets, which makes it lucrative for loggers to open-up even remote wilderness areas at high transportation costs. Mechanized extraction of mahogany and other prime timber species impacts the forest by creating canopy gaps and imparting much collateral damage due to logging roads and skid trails (Grogan et al.
2008). Mahogany and other high-value tropical timber species worldwide share several traits that predispose them to commercial extirpation: excellent pliable wood of exceptional beauty; natural distributions in forests experiencing rapid conversion rates; low-density populations
(often <1 tree/ha); and life histories generally characterized as non-pioneer late secondary, with fast growth rates, abiotic seed dispersal, and low-density seedlings requiring canopy disturbance for optimal seedling regeneration in the understory (Swaine and Whitmore 1988; Sodhi et al. 2008). One of the major obstacles to implementing a sustainable forestry sector in tropical countries is the lack of financial incentives for producers to limit offtakes to sustainable levels and invest in regeneration.

             Economic logic often dictates that trees should be felled whenever their rate of volume increment drops below the prevailing interest rate (Pearce 1990). Postponing harvest beyond this point would incur an opportunity cost because profits from logging could be invested at a higher rate elsewhere. This partly explains why many slow-growing timber species from tropical forests and savannahs are harvested unsustainably (e.g. East African Blackwood (Dalbergia melanoxylon) in the Miombo woodlands of Tanzania; Ball 2004). This is particularly the case where land tenure systems are unstable, and where there are no disincentives against ‘hit-and-run’ operations that mine the resource capital at one site and move on to undepleted areas elsewhere. This is clearly shown in a mahogany study in Bolivia where the smallest trees felled are ~40 cm in diameter, well below the legal minimum size (Gullison 1998). At this size, trees are increasing in volume at about 4% per year, whereas real mahogany price increases have averaged at only 1%, so that a 40-cm mahogany tree increases in value at about 5% annually, slowing down as the tree becomes larger. In contrast, real interest rates in Bolivia and other tropical countries are often >10%, creating a strong economic incentive to liquidate all trees of any value regardless of resource ownership.

Share

Twitter Delicious Facebook Digg Stumbleupon Favorites More