Henry David Thoreau

Thank God men cannot fly, and lay waste the sky as well as the earth.

Mohandas K. Gandhi

There is a sufficiency in the world for man's need but not for man's greed.

Robert Orben

There's so much pollution in the air now that if it weren't for our lungs there'd be no place to put it all.

Alan M. Eddison

Modern technology,Owes ecology,An apology.

Henrik Tikkanen

Because we don't think about future generations, they will never forget us.

Showing posts with label book. Show all posts

Saturday, June 1, 2013

Hunting and plant community dynamics


        Although the direct impacts of defaunation driven by overhunting can be predicted to some degree, higher-order indirect effects on community structure remain poorly understood since Redford’s (1992) seminal paper and may have profound, long-term consequences for the persistence of other taxa, and the structure, productivity and resilience of terrestrial ecosystems (Cunningham et al. 2009). Severe population declines or extirpation of the world’s megafauna may result in dramatic changes to ecosystems, some of which have already been empirically demonstrated, while others have yet to be documented or remain inexact. Large vertebrates often have a profound impact on food webs and community dynamics through mobile-linkage mutualisms, seed predation, and seedling and sapling herbivory. Plant communities in tropical forests depleted of their megafauna may experience pollinationbottlenecks, reduced seed dispersal, monodominance of seedling cohorts, altered patterns of seedling recruitment, other shifts in the relative abundance of species, and various forms of functional compensation (Cordeiro and Howe 2003; Peres and Roosmalen 2003; Wang et al. 2007; Terborgh et al. 2008; Chapter 3). On the other hand, the net effects of large mammal defaunation depends on how the balance of interactions are affected by population declines in both mutualists (e.g. highquality seed dispersers) and herbivores (e.g. seed predators) (Wright 2003). For example, significant changes in population densities in wild pigs (Suidae) and several other ungulates and rodents, which are active seed predators, may have a major effect on seed and seedling survival and forest regeneration (Curran and Webb 2000). 

               Tropical forest floras are most dependent on large-vertebrate dispersers, with as many as 97% of all tree, woody liana and epiphyte species bearing fruits and seeds that are morphologically adapted to endozoochorous (passing through the gut of an animal) dispersal (Peres and Roosmalen 2003). Successful seedling recruitment in many flowering plants depends on seed dispersal services provided by large-bodied frugivores (Howe and Smallwood 1982), while virtually all seeds falling underneath the parent’s canopy succumb to density-dependent mortality—caused by fungal attack, other pathogens, and vertebrate and invertebrate seed predators (see review in Carson et al. 2008). A growing number of phytodemographic studies have examined the effects of large-vertebrate removal. Studies examining seedling recruitment under different levels of hunting pressure (or disperser abundance) reveal very different outcomes. At the community level, seedling density in overhunted forests can be indistinguishable, greater, or less than that in the undisturbed forests (Dirzo and Miranda 1991; Chapman and Onderdonk 1998; Wright et al. 2000), but the consequences of increased hunting pressure to plant regeneration depends on the patterns of depletion across different prey species. In persistently hunted Amazonian forests, where large-bodied primates are driven to local extinction or severely reduced in numbers (Peres and Palacios 2007), the probability of effective dispersal of largeseeded endozoochorous plants can decline by over 60% compared to non-hunted forests (Peres and Roosmalen 2003). Consequently, plant species with seeds dispersed by vulnerable game species are less abundant where hunters are active, whereas species with seeds dispersed by abiotic means or by small frugivores ignored by hunters are more abundant in the seedling and sapling layers (Nuñez-Iturri and Howe 2007; Wright et al. 2007; Terborgh et al. 2008). 

                However, the importance of dispersal- limitation in the absence of large frugivores depends on the degree to which their seed dispersal services are redundant to any given plant species (Peres and Roosmalen 2003). Furthermore, local extinction events in large-bodied species are rarely compensated by smaller species in terms of their population density, biomass, diet, and seed handling outcomes (Peres and Dolman 2000). Large vertebrates targeted by hunters often have a disproportionate impact on community structure and operate as “ecosystem engineers” (Jones et al. 1994; Wright and Jones 2006), either performing a key landscaping role in terms of structural habitat disturbance, or as mega-herbivores that maintain the structure and relative abundance of plant communities. For example, elephants exert a major role in modifying vegetation structure and composition as herbivores, seed dispersers, and agents of mortality for many small trees (Cristoffer and Peres 2003). Two similar forests with or without elephants show different succession and regeneration pathways, as shown by long-term studies in Uganda (Sheil and Salim 2004). Overharvesting of several other species holding a keystone landscaping role can lead to pervasive changes in the structure and function of ecosystems. For example, the decimation of North American beaver populations by pelt hunters following the arrival of Europeans profoundly altered the hydrology, channel geomorphology, biogeochemical pathways and community productivity of riparian habitats (Naiman et al. 1986). Mammal overhunting triggers at least two additional potential cascades: the secondary extirpation of dependent taxa and the subsequent decline of ecological processes mediated by associated species. For instance, overhunting can severely disrupt key ecosystem processes including nutrient recycling and secondary seed dispersal exerted by relatively intact assemblages of dung beetles (Coleoptera: Scarabaeinae) and other coprophagous invertebrates that depend on large mammals for adult and larval food resources (Nichols et al. 2009).

Wednesday, April 3, 2013

Tropical forest disturbance


                Timber extraction in tropical forests is widely variable in terms of species selectivity, but even highly selective logging can trigger major ecological changes in the understory light environment, forest microclimate, and dynamics of plant regeneration. Even reduced-impact logging (RIL) operations can generate enough forest disturbance, through elevated canopy gap fracture, to greatly augment forest understory desiccation, dry fuel loads, and fuel continuity, thereby breaching the forest flammability threshold in seasonally-dry forests. During severe dry seasons, often aggravated by increasingly frequent continental- scale climatic events, extensive ground fires initiated by either natural or anthropogenic sources of ignition can result in a dramatically reduced biomass and biodiversity value of previously unburnt tropical forests (Barlow and Peres 2004, 2008). Despite these undesirable effects, large-scale commercial logging that is unsustainable at either the population or ecosystem level continues unchecked in many tropical forest frontiers (Curran et al. 2004; Asner et al. 2005). Yet surface fires aggravated by logging disturbance represent one of the most powerful mechanisms of functional and compositional impoverishment of remaining areas of tropical forests (Cochrane 2003), and arguably the most important climatemediated phase shift in the structure of tropical ecosystems

Thursday, December 13, 2012

Cascading effects of overexploitation on ecosystems

         
              All extractive systems in which the over harvested resource is one or more biological populations, can lead to pervasive trophic cascades and other unintended ecosystem-level consequences to non-target species. Most hunting, fishing, and collecting activities affect not only the primary target species, but also species that are taken accidentally or opportunistically. Furthermore, exploitation often causes physical damage to the environment, and has ramifications for other species through cascading interactions and changes in food webs. In addition, overexploitation may severely erode the ecological role of resource populations in natural communities. In other words, overexploited populations need not be entirely extirpated before they become ecologically extinct. In communities that are “half-empty” (Redford and Feinsinger 2001), populations may be reduced to sufficiently low numbers so that, although still present in the community, they no longer interact significantly with other species (Estes et al. 1989). Communities with reduced levels of species interactions may become pale shadows of their former selves. 

              Although difficult to measure, severe declines in large vertebrate populations may result in multi-trophic cascades that may profoundly alter the structure of marine ecosystems such as kelp forests, coral reefs and estuaries (Jackson et al. 2001), and analogous processes may occur in many terrestrial ecosystems. Plant reproduction in endemic island floras can be severely affected by population declines in flying foxes (pteropodid fruit bats) that serve as strong mutualists as pollinators and seed dispersers (Cox et al. 1991). In some Pacific archipelagos, several species may become functionally extinct, ceasing to effectively disperse large seeds long before becoming rare (McConkey and Drake 2006). A key agenda for future research will involve understanding the non-linearities between functional responses to the numeric abundance of strong interactors reduced by exploitation pressure and the quality of ecological services that depleted populations can perform. For example, what is the critical density of any given exploited population below which it can no longer fulfill its community-wide ecological role? 

                 In this section I concentrate on poorly known interaction cascades in tropical forest and marine environments, and discuss a few examples of how apparently innocuous extractive activities targeted to one or a few species can drastically affect the structure and functioning of these terrestrial and aquatic ecosystems.

Sunday, October 14, 2012

Overexploitation in aquatic ecosystems

              Marine biodiversity loss, largely through overfishing, is increasingly impairing the capacity of the world’s oceans to provide food, maintain water quality, and recover from perturbations (Worm et al. 2006). Yet marine fisheries provide employment and income for 0.2 billion people around the world, and fishing is the mainstay of the economy of many coastal regions; 41 million people worked as fishers or fish farmers in 2004, operating 1.3 million decked vessels and 2.7 million open boats (FAO 2007). An estimated 14 million metric tons of fuel was consumed by the fish-catching sector at a cost equivalent to US$22 billion, or ~25% of the total revenue of the sector. In 2004, reported catches from marine and inland capture fisheries were 85.8 million and 9.2 million tons, respectively, which was worth US$84.9 billion at first sale. Freshwater catches taken every year for food have declined recently but on average 500 000 tons are taken from the Mekong river in South-East Asia; 210 000 tons are taken from the Zaire river in Africa; and 210 000 tons of fish are taken from the Amazon river in South America. Seafood consumption is still high and rising in the First World and has doubled in China within the last decade. Fish contributes to, or exceeds 50% of the total animal protein consumption in many countries and regions, such as Bangladesh, Cambodia, Congo, Indonesia, Japan or the Brazilian Amazon. Overall, fish provides more than 2.8 billion people with ~20% or more of their average per capita intake of animal protein. 

             The oscillation of good and bad years in marine fisheries can also modulate the protein demand from terrestrial wildlife populations (Brashares et al. 2004). The share of fish in total world animal protein supply amounted to 16% in 2001 (FAO 2004). These ‘official’ landing statistics tend to severely underestimate catches and total values due to the enormous unrecorded contribution of subsistence fisheries consumed locally. Although the world’s oceans are vast, most seascapes are relatively low-productivity, and 80% of the global catch comes from only ~20% of the area. Approximately 68% of the world’s catch comes from the Pacific and northeast Atlantic. At current harvest rates, most of the economically important marine fisheries worldwide have either collapsed or are expected to collapse. Current impacts of overexploitation and its consequences are no longer locally nested, since 52% of marine stocks monitored by the FAO in 2005 were fully exploited at their maximum sustainable level and 24% were overexploited or depleted, such that their current biomass is much lower than the level that would maximize their sustained yield (FAO 2007). The remaining onequarter of the stocks were either underexploited or moderately exploited and could perhaps produce more. The Brazilian sardine (Sardinella brasiliensis) is a classic case of an overexploited marine fishery. In the 1970s hey-day of this industry, 200 000 tons were captured in southeast Brazil alone every year, but landings suddenly plummeted to <20 000 tons by 2001. Despite new fishing regulations introduced following its collapse, it is unclear whether southern Atlantic sardine stocks have shown any sign of recovery.

             With the possible exception of herring and related species that mature early in life and are fished with highly selective equipment, many gadids (e.g. cod, haddock) and other non-clupeids (e.g. flatfishes) have experienced little, if any, recovery in as much as 15 years after 45–99% reductions in reproductive biomass (Hutchings 2000). Worse still, an analysis of 147 populations of 39 wild fish species concluded that historically overexploited species, such as North Sea herring, became more prone to extreme year-on-year variation in numbers, rendering them vulnerable to economic or demographic extinction (Minto et al. 2008). Marine fisheries are an underperforming global asset—yields could be much greater if they were properly managed. The difference between the potential and actual net economic benefits from marine fisheries is in the order of US$50 billion per year—equivalent to over half thevalue of the global seafood trade (World Bank 2008). The cumulative economic loss to the global economy over the last three decades is estimated to be approximately US$2 trillion, and in many countries fishing operations are buoyed up by subsidies, so that the global fishery economy to the point of landing is already in deficit. Commercial fishing activities disproportionately threaten large-bodied marine and freshwater species (Olden et al. 2007). This results in fishermen fishing down the food chain, targeting ever-smaller pelagic fish as they can no longer capture top predatory fish. This is symptomatic of the now widely known process of ‘fishing down marine food webs’. Such sequential
size-graded exploitation systems also take place in multi-species assemblages hunted in tropical forests (Jerozolimski and Peres et al 2003). 

               In the seas, overexploitation threatens the persistence of ecologically significant populations of many large marine vertebrates, including sharks, tunas and sea turtles. Regional scale populations of large sharks worldwide have declined by 90% or more, and rapid declines of >75% of the coastal and oceanic Northwest Atlantic populations of scalloped hammerhead, white, and thresher sharks have occurred in the past 15 years (Baum et al. 2003; Myers and Worm 2003; Myers et al. 2007). Much of this activity is profligate and often driven by the surging global demand for shark fins. For example, in 1997 line fishermen captured 186 000 sharks in southern Brazil alone, of which 83% were killed and discarded in open waters following the removal of the most lucrative body parts (C.M. Vooren, pers. comm.). Of the large-bodied coastal species affected by this trade, several have virtually disappeared from shallow waters (e.g. greynurse sharks, Carcharias taurus). Official figures show that 131 tons of shark fins, corresponding to US $2.4 million, were exported from Brazil to Asia in 2007. Finally, we know rather little about ongoing extinction processes caused by harvesting. For example, from a compilation of 133 local, regional and global extinctions of marine fish populations, Dulvy et al. (2003) uncovered that exploitation was the main cause of extinctions (55% of all populations), but these were only reported after a median 53-year lag following their real-time disappearance. Some 80% of all extinctions were only discovered through historical comparisons; e.g. the near-extinction of large skates on both sides of the Atlantic was only brought to the world’s attention several decades after the declines have occurred.

Tuesday, September 18, 2012

Non-timber forest products

              Non-timber forest products (NTFPs) are biological resources other than timber which are extracted from either natural or managed forests (Peters 1994). Examples of exploited plant products include fruits, nuts, oil seeds, latex, resins, gums, medicinal plants, spices, dyes, ornamental plants, and raw materials such as firewood, Desmoncus climbing palms, bamboo and rattan. The socio-economic importance of NTFP harvest to indigenous peoples cannot be underestimated. Many ethnobotanical studies have catalogued the wide variety of useful plants (or plant parts) harvested by different aboriginal groups throughout the tropics. For example, the Waimiri-Atroari Indians of central Amazonia make use of 79% of the tree species occurring in a single 1 ha terra firme forest plot (Milliken et al. 1992), and 1748 of the ~8000 angiosperm species in the Himalayan region spanning eight Asian countries are used medicinally and many more for other purposes (Samant et al. 1998). Exploitation of NTFPs often involves partial or entire removal of individuals from the population, but the extraction method and whether vital parts are removed usually determine the mortality level in the exploited population. Traditional NTFP extractive practices are often hailed as desirable, low-impact economic activities in tropical forests compared to alternative forms of land use involving structural disturbance such as selective logging and shifting agriculture (Peters et al. 1989). As such, NTFP exploitation is usually assumed to be sustainable and a promising compromise between biodiversity conservation and economic development under varying degrees of market integration. The implicit assumption is that traditional methods of NTFP exploitation have little or no impact on forest ecosystems and tend to be sustainable because they have been practiced over many generations. However, virtually any form of NTFP exploitation in tropical forests has an ecological impact.

             The spatial extent and magnitude of this impact dependson the accessibility of the resource stock, the floristic composition of the forest, the nature and intensity of harvesting, and the particular species or plant part under exploitation. Yet few studies have quantitatively assessed the demographic viability of plant populations sourcing NTFPs. One exception are Brazil nuts (Bertholletia excelsa, Lecythidaceae) which comprise the most important wild seed extractive industry supporting millions of Amazonian forest dwellers for either subsistence or income. This wild seed crop is firmly established in export markets, has a history of 200 years of commercial exploitation, and comprises one of the most valuable non-timber extractive industries in tropical forests anywhere. Yet the persistent collection of B. excelsa seeds has severely undermined the patterns of seedling recruitment of Brazil nut trees. This has drastically affected the age structure of many natural populations to the point where persistently overexploited stands have succumbed to a process of senescence and demographic collapse, threatening this cornerston of the Amazonian extractive economy (Peres et al. 2003). A boom in the use of homeopathic remedies sustained by over collecting therapeutic and aromatic plants is threatening at least 150 species of European wild flowers and plants and driving many populations to extinction (Traffic 1998). Commercial exploitation of the Pau-Rosa or rosewood tree (Aniba rosaeodora, Lauraceae), which contains linalol, a key ingredient in luxury perfumes, involves a one-off destructive harvesting technique that almost invariably kills the tree. This species has consequently been extirpated from virtually its entire range in Brazilian Amazonia (Mitja and Lescure 2000). Channel 5 and other perfumes made with Pau-Rosa fragrance gained wide market demand decades ago, but
the number of processing plants in Brazil fell from 103 in 1966 to fewer than 20 in 1986, due to the dwindling resource base. Yet French perfume connoisseurs have been reluctant to accept replacing the natural Pau-Rosa fragrance with
synthetic substitutes, and the last remaining populations of Pau-Rosa remain threatened. 


              The same could be argued for a number of NTFPs for which the harvest by destructive practices involves a lethal injury to whole reproductive individuals. What then is the impact of NTFP extraction on the dynamics of natural populations? How does the impact vary with the life history of plants and animals harvested? Are current extraction rates truly sustainable? These are key questions in terms of the demographic sustainability of different NTFP offtakes, which will ultimately depend on the ability of the resource population to recruit new seedlings either continuously or in sporadic pulses while being subjected to a repeated history of exploitation. Unguarded enthusiasm for the role of NTFP exploitation in rural development partly stems from unrealistic economic studies reporting high market values. For example, Peters et al. (1989) reported that the net-value of fruit and latex extraction in the Peruvian Amazon was US$6330/ ha. This is in sharp contrast with a Mesoamerican study that quantified the local value of foods, construction materials, and medicines extracted from the forest by 32 indigenous Indian households (Godoy et al. 2000). The combined value of consumption and sale of forest goods ranged from US$18 to US$24 ha 1 yr 1, at the lower end of previous estimates (US$49 - US$1 089 ha 1 yr 1). NTFP extraction thus cannot be seen as a panacea for rural development and in many studies the potential value of NTFPs is exaggerated by unrealistic assumptions of high discount rates, unlimited market demands, availability of transportation facilities and absence of product substitution.

Sunday, September 2, 2012

Tropical forest vertebrates

             Humans have been hunting wildlife in tropical forests for over 100 000 years, but the extent of consumption has greatly increased over the last few decades. Tropical forest species are hunted for local consumption or sales in distant markets as food, trophies, medicines and pets. Exploitation of wild meat by forest dwellers has increased due to changes in hunting technology, scarcity of alternative protein, larger numbers of consumers, and greater access infrastructure. Recent estimates of the annual wild meat harvest are 23 500 tons in Sarawak (Bennett 2002), up to 164 692 tons in the Brazilian Amazon (Peres 2000), and up to 3.4 million tons in Central Africa (Fa and Peres 2001).
Hunting rates are already unsustainably high across vast tracts of tropical forests, averaging sixfold the maximum sustainable harvest in Central Africa (Fa et al. 2001). Consumption is both by rural and urban communities, who are often at the end of long supply chains that extend into many remote areas (Milner-Gulland et al. 2003). 


               The rapid acceleration in tropical forest defaunation due to unsustainable hunting initially occurred in Asia (Corlett 2007), is now sweeping through Africa, and is likely to move into the remotest parts of the neotropics (Peres and Lake 2003), reflecting human demographics in different continents. Hunting for either subsistence or commerce can profoundly affect the structure of tropical forest vertebrate assemblages, as revealed by both village- based kill-profiles (Jerozolimski and Peres 2003; Fa et al. 2005) and wildlife surveys in hunted and unhunted forests. This can be seen in the residual game abundance at forest sites subjected to varying degrees of hunting pressure, where overhunting often results in faunal biomass collapses, mainly through declines and local extinctions of large-bodied species (Bodmer 1995; Peres 2000). Peres and Palacios (2007) provide the first systematic estimates of the impact of hunting on the abundances of a comprehensive set of 30 reptile, bird, and mammal species across 101 forest sites scattered widely throughout the Amazon Basin and Guianan Shield. Considering the 12 most harvest sensitive species, mean aggregate population biomass was reduced almost eleven-fold from 979.8 kg/km2 in unhunted sites to only 89.2 kg/km2 in heavily hunted sites. 

              In KilumIjim, Cameroon, most large mammals, including elephants, buffalo, bushbuck, chimpanzees, leopards, and lions, have been lost as a result of hunting (Maisels et al. 2001). In Vietnam, 12 large vertebrate species have become virtually extinct over the last five decades primarily due to hunting (Bennett and Rao 2002). Pangolins and several other forest vertebrate species are facing regionalscale extinction throughout their range across southern Asia [Corlett 2007, TRAFFIC (The Wildlife Trade Monitoring Network) 2008], largely as a result of trade, and over half of all Asian freshwater turtle species are considered Endangered due to over-harvesting (IUCN 2007). In sum, game harvest studies throughout the tropics have shown that most unregulated, commercial hunting for wild meat is unsustainable (Robinson and Bennett 2000; Nasi et al. 2008), and that even subsistence hunting driven by local demand can severely threaten many medium to large-bodied vertebrate populations, with potentially far-reaching consequences to other species. However, persistent harvesting of multi-species prey assemblages can often lead to post-depletion equilibrium conditions in which slow-breeding, vulnerable taxa are eliminated and gradually replaced by fast-breeding robust taxa that are resilient to typical offtakes. For example, hunting in West African forests could now be defined as sustainable from the viewpoint of
urban bushmeat markets in which primarily rodents and small antelopes are currently traded, following a series of historical extinctions of vulnerable prey such as primates and large ungulates (Cowlishaw et al. 2005).

Sunday, August 12, 2012

Overexploitation in tropical forests

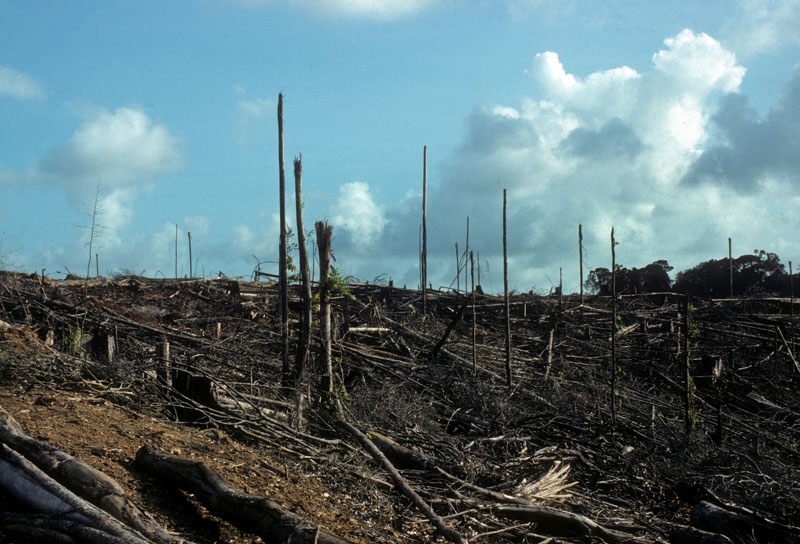
             Tropical deforestation is driven primarily by frontier expansion of subsistence agriculture and large development programs involving resettlement, agriculture, and infrastructure. However, animal and plant population declines are typically pre-empted by hunting and logging activity well before the coup de grâce of deforestation is delivered. It is estimated that between 5 and 7 million hectares of tropical forests are logged annually, approximately 68-79% of the area that was completely deforested each year between 1990 and 2005 [FAO (Food and Agriculture Organization of the United Nations) 2007]. Tropical forests account for ~25% of the global industrial wood production worth US$400 billion or ~2% of the global gross domestic product [WCFSD (World Commission on Forests and Sustainable Development) 1998]. Much of this logging activity opens up new frontiers to wildlife and non-timber resource exploitation, and catalyses the transition into a landscape dominated by slash-and burn and large-scale agriculture. Few studies have examined the impacts of selective logging on commercially valuable timber species and comparisons among studies are limited because they often fail to employ comparable methods that are adequately reported. The best case studies come from the most valuable timber species that have already declined in much of their natural ranges.

            For instance, the highly selective, but low intensity logging of broadleaf mahogany (Swietenia macrophylla), the most valuable widely traded Neotropical timber tree, is driven by the extraordinarily high prices in international markets, which makes it lucrative for loggers to open-up even remote wilderness areas at high transportation costs. Mechanized extraction of mahogany and other prime timber species impacts the forest by creating canopy gaps and imparting much collateral damage due to logging roads and skid trails (Grogan et al. 2008). Mahogany and other high-value tropical timber species worldwide share several traits that predispose them to commercial extirpation: excellent pliable wood of exceptional beauty; natural distributions in forests experiencing rapid conversion rates; low-density populations (often <1 tree/ha); and life histories generally characterized as non-pioneer late secondary, with fast growth rates, abiotic seed dispersal, and low-density seedlings requiring canopy disturbance for optimal seedling regeneration in the understory (Swaine and Whitmore 1988; Sodhi et al. 2008). One of the major obstacles to implementing a sustainable forestry sector in tropical countries is the lack of financial incentives for producers to limit offtakes to sustainable levels and invest in regeneration. Economic logic often dictates that trees should be felled whenever their rate of volume
increment drops below the prevailing interest rate (Pearce 1990). Postponing harvest beyond this point would incur an opportunity cost because profits from logging could be invested at a higher rate elsewhere.

            This partly explains why many slow-growing timber species from tropical forests and savannahs are harvested unsustainably (e.g. East African Blackwood (Dalbergia melanoxylon) in the Miombo woodlands of Tanzania; Ball 2004). This is particularly the case where land tenure systems are unstable, and where there are no disincentives against ‘hit-and-run’ operations that mine the resource capital at one site and move on to undepleted areas elsewhere. This is clearly shown in a mahogany study in Bolivia where the smallest trees felled are ~40 cm in diameter, well below the legal minimum size (Gullison 1998). At this size, trees are increasing in volume at about 4% per year, whereas real mahogany price increases have averaged at only 1%, so that a 40-cm mahogany tree increases in value at about 5% annually, slowing down as the tree becomes larger. In contrast, real interest rates in Bolivia and other tropical countries are often >10%, creating a strong economic incentive to liquidate all trees of any value regardless of resource ownership. Tropical deforestation is driven primarily by frontier expansion of subsistence agriculture and large development programs involving resettlement, agriculture, and infrastructure. However, animal and plant population declines are typically pre-empted by hunting and logging activity well before the coup de grâce of deforestation is delivered.

            It is estimated that between 5 and 7 million hectares of tropical forests are logged annually, approximately 68-79% of the area that was completely deforested each year between 1990 and 2005 [FAO (Food and Agriculture Organization of the United Nations) 2007]. Tropical forests account for ~25% of the global industrial wood production worth US$400 billion or ~2% of the global gross domestic product [WCFSD (World Commission on Forests and Sustainable Development) 1998]. Much of this logging activity opens up new frontiers to wildlife and non-timber resource exploitation, and catalyses the transition into a landscape dominated by slash-andburn and large-scale agriculture. Few studies have examined the impacts of selective logging on commercially valuable timber species and comparisons among studies are limited because they often fail to employ comparable methods that are adequately reported. The best case studies come from the most valuable timber species that have already declined in much of their natural ranges. For instance, the highly selective, but low intensity logging of broadleaf mahogany (Swietenia macrophylla), the most valuable widely traded Neotropical timber tree, is driven by the extraordinarily high prices in international markets, which makes it lucrative for loggers to open-up even remote wilderness areas at high transportation costs. Mechanized extraction of mahogany and other prime timber species impacts the forest by creating canopy gaps and imparting much collateral damage due to logging roads and skid trails (Grogan et al.
2008). Mahogany and other high-value tropical timber species worldwide share several traits that predispose them to commercial extirpation: excellent pliable wood of exceptional beauty; natural distributions in forests experiencing rapid conversion rates; low-density populations
(often <1 tree/ha); and life histories generally characterized as non-pioneer late secondary, with fast growth rates, abiotic seed dispersal, and low-density seedlings requiring canopy disturbance for optimal seedling regeneration in the understory (Swaine and Whitmore 1988; Sodhi et al. 2008). One of the major obstacles to implementing a sustainable forestry sector in tropical countries is the lack of financial incentives for producers to limit offtakes to sustainable levels and invest in regeneration.

             Economic logic often dictates that trees should be felled whenever their rate of volume increment drops below the prevailing interest rate (Pearce 1990). Postponing harvest beyond this point would incur an opportunity cost because profits from logging could be invested at a higher rate elsewhere. This partly explains why many slow-growing timber species from tropical forests and savannahs are harvested unsustainably (e.g. East African Blackwood (Dalbergia melanoxylon) in the Miombo woodlands of Tanzania; Ball 2004). This is particularly the case where land tenure systems are unstable, and where there are no disincentives against ‘hit-and-run’ operations that mine the resource capital at one site and move on to undepleted areas elsewhere. This is clearly shown in a mahogany study in Bolivia where the smallest trees felled are ~40 cm in diameter, well below the legal minimum size (Gullison 1998). At this size, trees are increasing in volume at about 4% per year, whereas real mahogany price increases have averaged at only 1%, so that a 40-cm mahogany tree increases in value at about 5% annually, slowing down as the tree becomes larger. In contrast, real interest rates in Bolivia and other tropical countries are often >10%, creating a strong economic incentive to liquidate all trees of any value regardless of resource ownership.

Saturday, December 10, 2011

Changes to ecosystem processes

              Removal of large tracts of native vegetation changes physical processes, such as those relating to solar radiation and the fluxes of wind and water (Saunders et al. 1991). The greatest impact on fragments occurs at their boundaries; small remnants and those with complex shapes experience the strongest “edge effects”. For example, the micro climate at a forest edge adjacent to cleared land differs from that of the forest interior in attributes such as incident light, humidity, ground and air temperature, and wind speed. In turn, these physical changes affect biological processes such as litter decomposition and nutrient cycling, and the structure and composition of vegetation. Changes to biophysical processes from land use in the surrounding environment, such as the use of fertilizers on farmland, alterations to drainage patterns and water flows, and the presence of exotic plants and animals, also have spill-over effects in fragments. 

               Many native vegetation communities are resistant to invasion by exotic plant species unless they are disturbed. Grazing by domestic stock and altered nutrient levels can facilitate the invasion of exotic species of plants, which markedly alters the vegetation in fragments (Hobbs and Yates 2003) and habitats for animals. The intensity of edge effects in fragments and the distance over which they act varies between processes and between ecosystems. In tropical forests in the Brazilian Amazon, for example, changes in soil moisture content, vapor pressure deficit, and the number of tree fall gaps extend about 50 m into the forest, whereas the invasion of disturbance-adapted butterflies and beetles and elevated tree mortality extend 200 m or more from the forest edge (Laurance 2008). 

               In most situations, changes at edges are generally detrimental to conservation values because they modify formerly intact habitats. However, in some circumstances edges are deliberately managed to achieve specific outcomes. Manipulation of edges is used to enhance the abundance of game species such as deer, pheasants and grouse. In England, open linear “rides” in woods may be actively managed to increase incident light and early succession habitat for butterflies and other wildlife (Ferris-Kaan 1995). Changes to biophysical processes frequently have profound effects for entire landscapes. 

              In highly fragmented landscapes in which most fragments are small or have linear shapes, there may be little interior habitat that is buffered from edge effects. Changes that occur to individualfragments accumulate across the landscape. Changes to biophysical processes such as hydrological regimes can also affect entire landscapes. In the Western Australian wheat belt, massive loss of native vegetation has resulted in a rise in the level of groundwater, bringing stored salt (NaCl) to the surface where it accumulates and reduces agricultural productivity and transforms native vegetation (Hobbs 1993).

Friday, November 25, 2011

Tropical and subtropical forests

               A second way to assess habitat loss is by contrastingmajor  biomes or ecosystem types. Today, tropical rainforests (also termed tropical moist and humid forests) are receiving the greatest attention, because they are being destroyed so rapidly and because they are the most biologically diverse of all terrestrial biomes. Of the roughly 16 million km2 of tropical rainforest that originally existed worldwide, less than 9 million km2 remains today (Whitmore 1997; MEA 2005). The current rate of rainforest loss is debated, with different estimates ranging from around 60 000 km2 (Achard et al. 2002) to 130 000 km2 per year (FAO 2000). Regardless of which estimate one adheres to, rates of rainforest loss are alarmingly high. Rates of rainforest destruction vary considerably among geographic regions. Of the world’s three major tropical regions, Southeast Asian forests are disappearing most rapidly in relative terms , while the African and New World tropics have somewhat lower rates of percent- annual forest loss (Sodhi et al. 2004). Such averages, however, disguise important smaller scale variation. 

               In the New World tropics, for example, the Caribbean, Meso American, and Andean regions are all suffering severe rainforest loss, but the relative deforestation rate for the region as a whole is buffered by the vastness of the Amazon. Likewise, in tropical Africa, forest loss is severe in West Africa, montane areas of East Africa, and Madagascar, but substantial forest still survives in the Congo Basin (Laurance 1999). Other tropical and subtropical biomes have suffered even more heavily than rainforests. Tropical dry forests (also known as monsoonal or deciduous forests) have been severely reduced, in part because they are easier to clear and burn than rainforests. For instance, along Central America’s Pacific coast, much less than 1% of the original dry forest survives. Losses of dry forest have been nearly as severe in Madagascar and parts of Southeast Asia (Laurance 1999; Mayaux et al. 2005).
 

                Mangrove forests, salt-tolerant ecosystems that grow in tropical and subtropical intertidal zones, have also been seriously reduced. Based on countries for which data exist, more than a third of all mangroves were lost in the last few decades of the 20th century (MEA 2005). From 1990 to 2000, over 1% of all mangrove forests were lost annually, with rates of loss especially high in Southeast Asia (Mayaux et al. 2005). Such losses are alarming given the high primary productivity of mangroves, their key role as spawning and rearing areas for economically important fish and shrimp species, and their importance for sheltering coastal areas from destructive storms and tsunamis (Danielsen et al. 2005).

Monday, November 21, 2011

Valuing Ecosystem Services

              Ecosystems and their constituent species provide an endless stream of products, functions, and services that keep our world running and make our existence possible. To many, even the thought of putting a price tag on services like photosynthesis, purification of water, and pollination of food crops may seem like hubris, as these are truly priceless services without which not only humans, but most of life would perish.A distinguished economist put it best in response to a seminar at the USA Federal Trade Commission, where the speaker downplayed the impact of global warming by saying agriculture and forestry “accounted for only three percent of the US gross national product”. The economist’s response was: “What does this genius think we’re going to eat?” (Naylor and Ehrlich 1997). Nevertheless, in our financially-driven world, we need to quantify the trade - offs involved in land use scenarios that maximize biodiversity conservation and ecosystem services versus scenarios that maximize profit from a single commodity. Without such assessments, special interests representing single objectives dominate the debate and sideline the integration of ecosystem services into the decision-making process (Nelson et al. 2009). 

               Valuing ecosystem services is not an end in itself, but is the first step towards integrating these services into public decision-making and ensuring the continuity of ecosystems that provide the services (Goulder and Kennedy 1997; National Research Council 2005; Daily et al. 2009). Historically, ecosystem services have been mostly thought of as free public goods, an approach which has too frequently led to the “tragedy of the commons” where vital ecosystem goods like clean water have been degraded and consumed to extinction (Daily 1997). Too often, ecosystem services have been valued, if at all, based on “marginal utility” (Brauman and Daily 2008). When the service (like cleanwater) is abundant, themarginal utility of one additional unit can be as low as zero. However, as the service becomes more scarce, the marginal utility of each additional unit becomes increasingly valuable (Goulder and Kennedy 1997). Using the marginal value for a service when it is abundant drastically underestimates the value of the service as it becomes scarcer. As Benjamin Franklin wryly observed, “When the well’s dry,we know the worth of water.” As the societal importance of ecosystem services becomes increasingly appreciated, there has been a growing realization that successful application of this concept requires a skilful combination of biological, physical, and social sciences, as well as the creation of new programs and institutions. 

              The scientific community needs to help develop the necessary quantitative tools to calculate the value of ecosystem services and to present them to the decision makers (Daily et al. 2009). A promising example is the InVEST (Integrated Valuation of Ecosystem Services and Tradeoffs) system (Daily et al. 2009; Nelson 2009) developed by the Natural Capital Project (www.naturalcapital.org). However, good tools are valuable only if they are used. A more difficult goal is convincing the private and public sectors to incorporate ecosystem services into their decision - making processes (Daily et al. 2009). Nevertheless, with the socio-economic impacts and human costs of environmental catastrophes, such as Hurricane Katrina, getting bigger and more visible, and with climate change and related carbon sequestration schemes having reached a prominent place in the public consciousness, the value of these services and the necessity of maintaining them has become increasingly mainstream. Recent market-based approaches such as payments for Costa Rican ecosystem services, wetland mitigation banks, and the Chicago Climate Exchange have proven useful in the valuation of ecosystem services (Brauman and Daily 2008). Even though the planet’s ecosystems, the biodiversity they harbor, and the services they collectively provide are truly priceless, market-based and other quantitative approaches for valuing ecosystem services will raise the profile of nature’s services in the public consciousness, integrate these services into decision-making, and help ensure the continuity of ecosystem contributions to the healthy functioning of our planet and its residents.

Saturday, November 19, 2011

Nature’s Cures versus Emerging Diseases

            While many people know about how plants prevent erosion, protect water supplies, and “clean the air”, how bees pollinate plants or how owls reduce rodent activity, many lesser-known organisms not only have crucial ecological roles, but also produce unique chemicals and pharmaceuticals that can literally save people’s lives. Thousands of plant species are used medically by traditional, indigenous communities worldwide. These peoples’ ethno botanical knowledge has led to the patenting, by pharmaceutical companies, of more than a quarter of all medicines (Posey 1999), although the indigenous communities rarely benefit from these patents (Mgbeoji 2006). Furthermore, the eroding of traditions worldwide, increasing emigration from traditional, rural communities to urban areas, and disappearing cultures and languages mean that the priceless ethno botanical knowledge of many cultures is rapidly disappearing in parallel with the impending extinctions of many medicinal plants due to habitat loss and over harvesting (Millennium Ecosystem Assessment 2005a). Some of the rainforest areas that are being deforested fastest, like the island of Borneo, harbor plant species that produce active anti-HIV (Human Immunodeficiency Virus) agents (Chung 1996; Jassim and Naji 2003). 

             Doubtlessly, thousands more useful and vital plant compounds await discovery in the forests of the world, particularly in the bio diverse tropics (Laurance 1999; Sodhi et al. 2007)however, without an effective strategy that integrates community based habitat conservation, rewarding of local ethno botanical knowledge, and scientific research on these compounds, many species, the local knowledge of them, and the priceless cures they offer will disappear before scientists discover them.

              As with many of nature’s services, there is a flip side to the medicinal benefits of biodiversity, namely, emerging diseases ( Jones et al. 2008). The planet’s organisms also include countless diseases, many of which are making the transition to humans as people increasingly invade the habitats of the hosts of these diseases and consume the hosts themselves. Three quarters of human diseases are thought to have their origins in domestic or wild animals and new diseases are emerging as humans increase their presence in formerly wilderness areas (Daily and Ehrlich 1996; Foley et al. 2005). Some of the deadliest diseases, such as monkey pox, malaria, HIV and Ebola, are thought to have initially crossed from central African primates to the people who hunted, butchered, and consumed them (Hahn et al. 2000; Wolfe et al. 2005; Rich et al. 2009). Some diseases emerge in ways that show the difficulty of predicting the consequences of disturbing ecosystems. The extensive smoke from the massive 1997–1998 forest fires in South east Asia is thought to have led to the fruiting failure of many forest trees, forcing frugivorous bats to switch to fruit trees in pig farms. The bats, which host the Nipah virus, likely passed it to the pigs, from which the virus made the jump to people (Chivian 2002). Another classic example from Southeast Asia is the Severe Acute Respiratory Syndrome (SARS). 

            So far having killed 774 people, the SARS coronavirus has been recently discovered in wild animals like the masked palm civet (Paguma larvata) and raccoon dog (Nyctereuteus procyonoides) that are frequently consumed by people in the region (Guan et al. 2003). SARS like corona viruses have been discovered in bats (Li et al. 2005) and the virus was probably passed to civets and other animals as they ate fruits partially eaten and dropped by those bats (Jamie H. Jones, personal communication). 

              It is probable that SARS made the final jump to people through such animals bought for food in wildlife markets. The recent emergence of the deadly avian influenza strain H5N1 provides another good example. Even though there are known to be at least 144 strains of avian flu, only a few strains kill people. However, some of the deadliest pandemics have been among these strains, including H1N1, H2N, and H3N2 (Cox and Subbarao 2000). H5N1, the cause of the recent bird flu panic, has a 50% fatality rate and may cause another human pandemic. At low host densities, viruses that become too deadly, fail to spread. It is likely that raising domestic birds in increasingly higher densities led to
the evolution of higher virulence in H5N1, as it became easier for the virus to jump to another host before it killed its original host. There is also a possibility that increased invasion of wilderness areas by people led to the jump of H5N1 from wild birds to domestic birds, but that is yet to be proven. Malaria, recently shown to have jumped from chimpanzees to humans (Rich et al. 2009), is perhaps the best example of a resurging disease that increases as a result of tropical deforestation (Singer and Castro 2001; Foley et al. 2005; Yasuoka and Levins 2007). 

               Pearson (2003) calculated that every 1% increase in deforestation in the Amazon leads to an 8% increase in the population of the malaria vector mosquito (Anopheles darlingi). In addition, some immigrants colonizing deforested areas brought new sources of malaria (Moran 1988) whereas other immigrants come from malaria-free areas and thus become ideal hosts with no immunity (Aiken and Leigh 1992). Collectively, the conditions leading to and resulting from tropical deforestation, combined with climate change, human migration, agricultural intensification, and animal trafficking create the perfect storm for the emergence of new diseases as well as the resurgence of old ones. In the face of rapid global change, ecologically intact and relatively stable communities may be our best weapon against the emergence of new diseases.

Monday, November 14, 2011

Biodiversity and Ecosystem Function

               The role of biodiversity in providing ecosystem services is actively debated in ecology. The diversity of functional groups (groups of ecologically equivalent species (Naeem and Li 1997)), is as important as species diversity, if not more so (Kremen 2005), and in most services a few dominant species seem to play the major role (Hooper et al. 2005). However, many other species are critical for eco system functioning and provide “insurance” against disturbance, environmental change, and the decline of the dominant species (Tilman 1997; Ricketts et al. 2004; Hobbs et al. 2007). As for many other ecological processes, it was Charles Darwin who first wrote of this, noting that several distinct genera of grasses grown together would produce more plants and more herbage than a single species growing alone (Darwin 1872). Many studies have confirmed that increased biodiversity improves ecosystem functioning in plant communities (Naeem and Li 1997; Tilman 1997). Different plant species capture different resources, leading to greater efficiency and higher productivity (Tilman et al. 1996). Due to the“sampling-competition effect” the presence of more species increases the probability of having a particularly productive species in any given environment (Tilman 1997). Furthermore, different species’ ecologies lead to complementary resource use, where each species grows best under a specific range of environmental conditions, and different species can improve environmental conditions for other species (facilitation effect; Hooper et al. 2005). Consequently, the more complex an ecosystem is, the more biodiversity will increase ecosystem function, as more species are needed to fully exploit the many combinations of environmental variables (Tilman 1997). More biodiverse ecosystems are also likely to be more stable and more efficient due to the presence of more pathways for energy flow and nutrient recycling (Macarthur 1955; Hooper et al. 2005; Vitousek and Hooper 1993; Worm et al. 2006). Greenhouse and field experiments have confirmed that biodiversity does increase ecosystem productivity, while reducing fluctuations in productivity (Naeem et al. 1995; Tilman et al. 1996). 

               Although increased diversity can increase the population fluctuations of individual species, diversity is thought to stabilize overall ecosystem functioning (Chapin et al. 2000; Tilman 1996) and make the ecosystem more resistant to perturbations (Pimm 1984). These hypotheses have been confirmed in field experiments, where speciesrich plots showed less yearly variation in productivity (Tilman 1996) and their productivity during a drought year declined much less than species poor plots (Tilman and Downing 1994). Because more species do better at utilizing and recycling nutrients, in the long-term, species-rich plots are
better at reducing nutrient losses and maintaining soil fertility (Tilman et al. 1996; Vitousek and Hooper 1993). Although it makes intuitive sense that the species that dominate in number and/or biomass are more likely to be important for ecosystem function (Raffaelli 2004; Smith et al. 2004), in some cases, even rare species can have a role, forexample, in increasing resistance to invasion (Lyons and Schwartz 2001). A keystone species is one that has an ecosystem impact that is disproportionately large in relation to its abundance (Hooper et al. 2005; Power et al. 1996;). Species that are not thought of as “typical” keystones can turn out to be so, sometimes in more ways than one (Daily et al. 1993). Even though in many communities only a few species have strong effects, the weak effects of many species can add up to a substantial stabilizing effect and seemingly “weak” effects over broad scales can be strong at the local level (Berlow 1999). Increased species richness can “insure” against sudden change, which is now a global phenomenon (Parmesan and Yohe 2003; Root et al. 2003). Even though a few species may make up most of the biomass of most functional groups, this does not mean that other species are
unnecessary (Walker et al. 1999). 

              Species may act like the rivets in an airplane wing, the loss of each unnoticed until a catastrophic threshold is passed (Ehrlich and Ehrlich 1981b). As humanity’s footprint on the planet increases and formerly stable ecosystems experience constant disruptions in the form of introduced species, pollution , climate change, excessive nutrient loads, fires, and many other perturbations, the insurance value of biodiversity has become increasingly vital over the entire range of habitats and systems, from diverse forest stands sequesterin CO2 better in the long-term (Bolker et al. 1995; Hooper et al. 2005; but see Tallis and Kareiva 2006) to forest-dwelling native bees’ coffee pollination services increasing coffee production in Costa Rica (Ricketts et al. 2004;). With accelerating losses of unique species, humanity, far from hedging its bets, is moving ever closer to the day when we will run out of options on an increasingly unstable planet.

Wednesday, November 9, 2011

Soils and Erosion

                 Without forest cover, erosion rates skyrocket, and many countries, especially in the tropics, lose astounding amounts of soil to erosion. Worldwide, 11 million km2 of land (the area of USA and Mexico combined) are affected by high rates of erosion (Millennium Ecosystem Assessment 2005b). Every year about 75 billion tons of soil are thought to be eroded from terrestrial ecosystems, at rates 13–40 times faster than the average rate of soil formation (Pimentel and Kounang 1998). Pimentel et al. (1995) estimated that in the second half of the 20th century about a third of the world’s arable land was lost to erosion. This means losing vital harvests and income (Myers 1997), not to mention losing lives to malnutrition and starvation. Soil is one of the most critical but also most underappreciated and abused elements of natural capital, one that can take a few years to lose and millennia to replace. A soil’s character is determined by six factors: topography, the nature of the parent material, the age of the soil, soil organisms and plants, climate, and human activity (Daily et al. 1997). For example, in the tropics, farming can result in the loss of half the soil nutrients in less than a decade (Bolin and Cook 1983), a loss that can take centuries to restore. In arid areas, the replacement of native deep rooted plants with shallow-rooted crop plants can lead to a rise in the water table, which can bring soil salts to the surface (salinization), cause water logging, and consequently result in crop losses (Lefroy et al. 1993). Soil provides six major ecosystem services (Daily et al. 1997):

  • Moderating the hydrologic cycle. 
  • Physical support of plants. 
  • Retention and delivery of nutrients to plants. 
  • Disposal of wastes and dead organic matter. 
  • Renewal of soil fertility. 
  • Regulation of major element cycles.
                Every year enough rain falls to cover the planet with one meter of water (Shiklomanov 1993), but thanks to soil’s enormous water retention capacity, most of this water is absorbed and gradually released to feed plants, underground aquifers, and rivers.However, intensive cultivation, by lowering soil’s organic matter content, can reduce this capacity, leading to floods, erosion, pollution, and further loss of organic matter (Pimentel et al. 1995). Soil particles usually carry a negative charge, which plays a critical role in delivering nutrient cations (positively-charged ions) like Ca2þ, Kþ, Naþ, NH4þ, and Mg2þ to plants (Daily et al. 1997). To deliver these nutrients without soil would be exceedingly expensive as modern hydroponic (water-based) systems cost more than US$250 000 per ha (Canada’s Office of Urban
Agriculture 2008; Avinash 2008). 

                Soil is also critical in filtering and purifying water by removing contaminants, bacteria, and other impurities (Fujii et al. 2001). Soils harbor an astounding diversity of microorganisms, including thousands of species of protozoa, antibiotic-producing bacteria (which produce streptomycin) and fungi (producing penicillin), as well as myriad invertebrates, worms and algae (Daily et al. 1997). These organisms play fundamental roles in decomposing dead matter, neutralizing deadly pathogens, and recycling waste into valuable nutrients. Just the nitrogen fixed by soil organisms like Rhizobium bacteria amounts to about 100 million metric tons per year (Schlesinger 1991). It would cost at least US$320 billon/year to replace natural nitrogen fertilization with fertilizers (Daily et al. 1997). As the accelerating release of CO2, N2O (Nitrous Oxide), methane and other greenhouse gases increasingly modifies climate (IPCC 2007), the soil’s capacity to store these molecules is becoming even more vital. Per area, soil stores 1.8 times the carbon and 18 times the nitrogen that plants alone can store (Schlesinger 1991). For peatlands, soil carbon storage can be 10 times greater than that stored by the plants growing on it and peatland fires release massive amounts of CO2 into the atmosphere (Page and Rieley 1998). Despite soil’s vital importance, 17% of the Earth’s vegetated land surface (Oldeman 1998) or 23% of all land used for food production
[FAO (Food and Agriculture Organization of the United Nations) 1990] has experienced soil degradation since 1945. Erosion is the best-known example of the disruption of the sedimentary cycle. 

                       Although erosion is responsible for releasing nutrients from bedrock and making them available to plants, excessive wind and water erosion results in the removal of top soil, the loss of valuable nutrients, and desertification. The direct costs of erosion total about US$250 billion per year and the indirect costs (e.g. siltation, obsolescence of dams, water quality declines) approximately $150 billion per year (Pimentel et al. 1995). Sufficient preventive measures would cost only 19% of this total (Pimentel et al. 1995). The loss of vegetative cover increases the erosional impact of rain. In intact forests, most rain water does not hit the ground directly and tree roots hold the soil together against being washed away (Brauman et al. 2007), better than in logged forest or plantations (Myers 1997) where roads can increase erosion rates (Bruijnzeel 2004). The expansion of farming and deforestation have doubled the amount of sediment discharged into the oceans. Coral reefs can experience high mortality after being buried by sediment discharge (Pandolfi et al. 2003; Bruno and Selig 2007). Wind erosion can be particularly severe in desert ecosystems, where even small increases in vegetative cover (Hupy 2004) and reduced tillage practices (Gomes et al. 2003) can lessen wind erosion substantially. Montane areas are especially prone to rapid erosion (Milliman and Syvitski 1992), and revegetation programs are critical in such ecosystems (Vanacker et al. 2007). Interestingly, soil carbon buried in deposits resulting from erosion, can produce carbon sinks that can offset up to 10% of the global fossil fuel emissions of CO2 (Berhe et al. 2007). 

                 However, erosion also lowers soil productivity and reduces the organic carbon returned to soil as plant residue (Gregorich et al. 1998). Increasing soil carbon capacity by 5–15% through soil-friendly tillage practices not only offsets fossil-fuel carbon emissions by a roughly equal amount but also increases crop yields and enhances food security (Lal 2004). An increase of one ton of soil carbon pool in degraded cropland soils may increase crop yield by 20 to 40 kilograms per ha (kg/ha) for wheat, 10 to 20 kg/ha for maize, and 0.5 to 1 kg/ha for cowpeas (Lal 2004).

Monday, November 7, 2011

Regulation of the Hydrologic Cycle

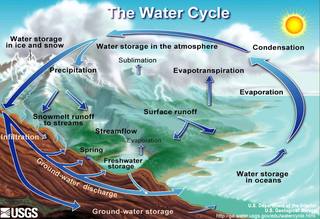
                One of the most vital and immediate services of ecosystems, particularly of forests, rivers and wetlands, is the provisioning and regulation of water resources. These services provide a vast range of benefits from spiritual to life-saving, illustrated by the classification of hydrologic services into five broad categories by Brauman et al. (2007): improvement of extractive water supply, improvement of in-stream water supply, water damage mitigation, provision of water-related cultural services, and water-associated supporting services. Although 71% of the planet is covered by water, most of this is seawater unfit for drinking or agriculture (Postel et al. 1996). Fresh water not locked away in glaciers and icecaps constitutes 0.77% of the planet’s water (Shiklomanov 1993). To provide sufficient fresh water to meet human needs via industrial desalination (removing the salt from seawater) would cost US$3 000 billion per year (Postel and Carpenter 1997). Quantity, quality, location, and timing of water provision determine the scale and impact of hydrologic services (Brauman et al. 2007). These attributes can make the difference between water as a blessing (e.g. drinking water) or a curse (e.g. floods). Water is constantly redistributed through the hydrologic cycle. Fresh water comes down as precipitation, collects in water bodies or is absorbed by the soil and plants. 

                 Some of the water flows unutilized into the sea or seeps intounderground aquifers where it can remain for millennia unless extracted by people; mining this “fossil” groundwater is often unsustainable and is a serious problem in desert regions like Libya (Millennium Ecosystem Assessment 2005c). The cycle is completed when water vapor is released back into the atmosphere either through evaporation from land and water bodies or by being released
from plants (transpiration) and other organisms. Rising environmental temperatures are expected to increase evaporation and consequent precipitation in some places and raise the likelihood of droughts and fires in other places, both scenarios that would have major consequences for the world’s vegetation (Wright 2005). These changes in turn can lead to further climatic problems, affecting agriculture and communities worldwide. Ecosystems, particularly forests, play major roles in the regulation of the hydrologic cycle and also have the potential to moderate the effects of climate change. Tropical forests act as heat and humidity pumps, transferring heat from the tropics to the temperate zones and releasing water vapor that comes back as rain (Sodhi et al. 2007). Extensive tropical deforestation is expected to lead to higher temperatures, reduced precipitation, and increased frequency of droughts and fires, all ofwhich are likely to reduce tropical forest cover in a positive feedback loop (Sodhi et al. 2007). Forest ecosystems alone are thought to regulate approximately a third of the planet’s watersheds on which nearly five billion people rely (Millennium Ecosystem Assessment 2005c). With increasing human population and consequent water pollution, fresh water is becoming an increasingly precious resource, especially in arid areas like the Middle East, where the scarcity of water is likely to lead to increasing local conflicts in the 21st century (Klare 2001; Selby 2005). 

                  Aquatic ecosystems, in addition to being vital sources of water, fish, waterfowl, reeds, and other resources, also moderate the local climate and can act as buffers for floods, tsunamis, and other water incursions. For example, the flooding following Hurricane Katrina would have done less damage if the coastal wetlands surrounding New Orleans had had their original extent (Day et al. 2007). The impact of the 24 December 2004 tsunami in Southeast Asia would have been reduced if some of the hardest hit areas had not been stripped of their mangrove forests (Dahdouh-guebas et al. 2005; Danielsen et al. 2005). These observations support analytical models in which thirty “waru” trees (Hibiscus tiliaceus) planted along a 100 m by 1 meter band reduced the impact of a tsunami by 90% (Hiraishi and Harada 2003), a solution more effective and cheaper than artificial barriers. Hydrologic regulation by ecosystems begins with the first drop of rain. Vegetation layers, especially trees, intercept raindrops, which gradually descend into the soil, rather than hitting it directly and leading to erosion and floods. By intercepting rainfall and promoting soil development, vegetation can modulate the timing of flows and potentially reduce flooding. Flood mitigation is particularly crucial in tropical areas where downpours can rapidly deposit enormous amounts of water that can lead to increased erosion, floods, and deaths if there is little natural forest to absorb the rainfall (Bradshaw et al. 2007). Studies of some watersheds have shown that native forests reduced flood risks only at small scales, leading some hydrologists to question directly connecting forest cover to flood reduction (Calder and Aylward 2006). However, in the first global-scale empirical demonstration that forests are correlated with flood risk and severity in developing countries, Bradshaw et al. (2007) estimated that a 10% decrease in natural forest area would lead to a flood frequency increase between 4% and 28%, and to a 4–8% increase in total flood duration at the country scale. 

                Compared to natural forests, however, afforestation programs or forest plantations may not reduce floods, or may even increase flood volume due to road construction, soil compaction, and changes in drainage regimes (Calder and Aylward 2006). Non-native plantations can do more harm than good, particularly when they reduce dry season water flows (Scott et al. 2005). Despite covering only 6% of the planet’s surface, tropical forests receive nearly half of the world’s rainfall, which can be as much as 22 500 mm during five months of monsoon season in India (Myers 1997). In Southeast Asia, an intact old-growth dipterocarp forest intercepts at least 35% of the rainfall, while a logged forest intercepts less than 20%, and an oil palm (Elaeis spp.) plantation intercepts only 12% (Ba 1977). As a consequence, primary forest can moderate seasonal extremes in water flow and availability better than more intensive land uses like plantation forestry and agriculture. For example, primary forest in Ivory Coast releases three to five times as much water at the end of the dry season compared to a coffee plantation (Dosso 1981). However, it is difficult to make generalizations about hydrologic response in the tropics. For example, local soil and rainfall patterns can result in a
65-fold variation in tropical natural sedimentation rates (Bruijnzeel 2004). This underlines the importance of site-specific studies in the tropics, but most hydrologic studies of ecosystems have taken place in temperate ecosystems (Brauman et al. 2007).

Share

Twitter Delicious Facebook Digg Stumbleupon Favorites More